Two new papers, one published today in Nature by Vadim Gladyshev and colleagues at Harvard, and a recent one in Cell by Juan Carlos Izpisua Belmonte and his team at Altos Labs, have provided a new model for the biology of aging, and what might be done to reverse it. Until recently we accepted that aging of cells was due to “wear and tear” like rusting out a car. The idea that accumulated damage is the principal pathway for cell aging is now complemented by the loss of cell identity model. We don’t know the relative contribution or interdependence of these 2 models in the aging process.
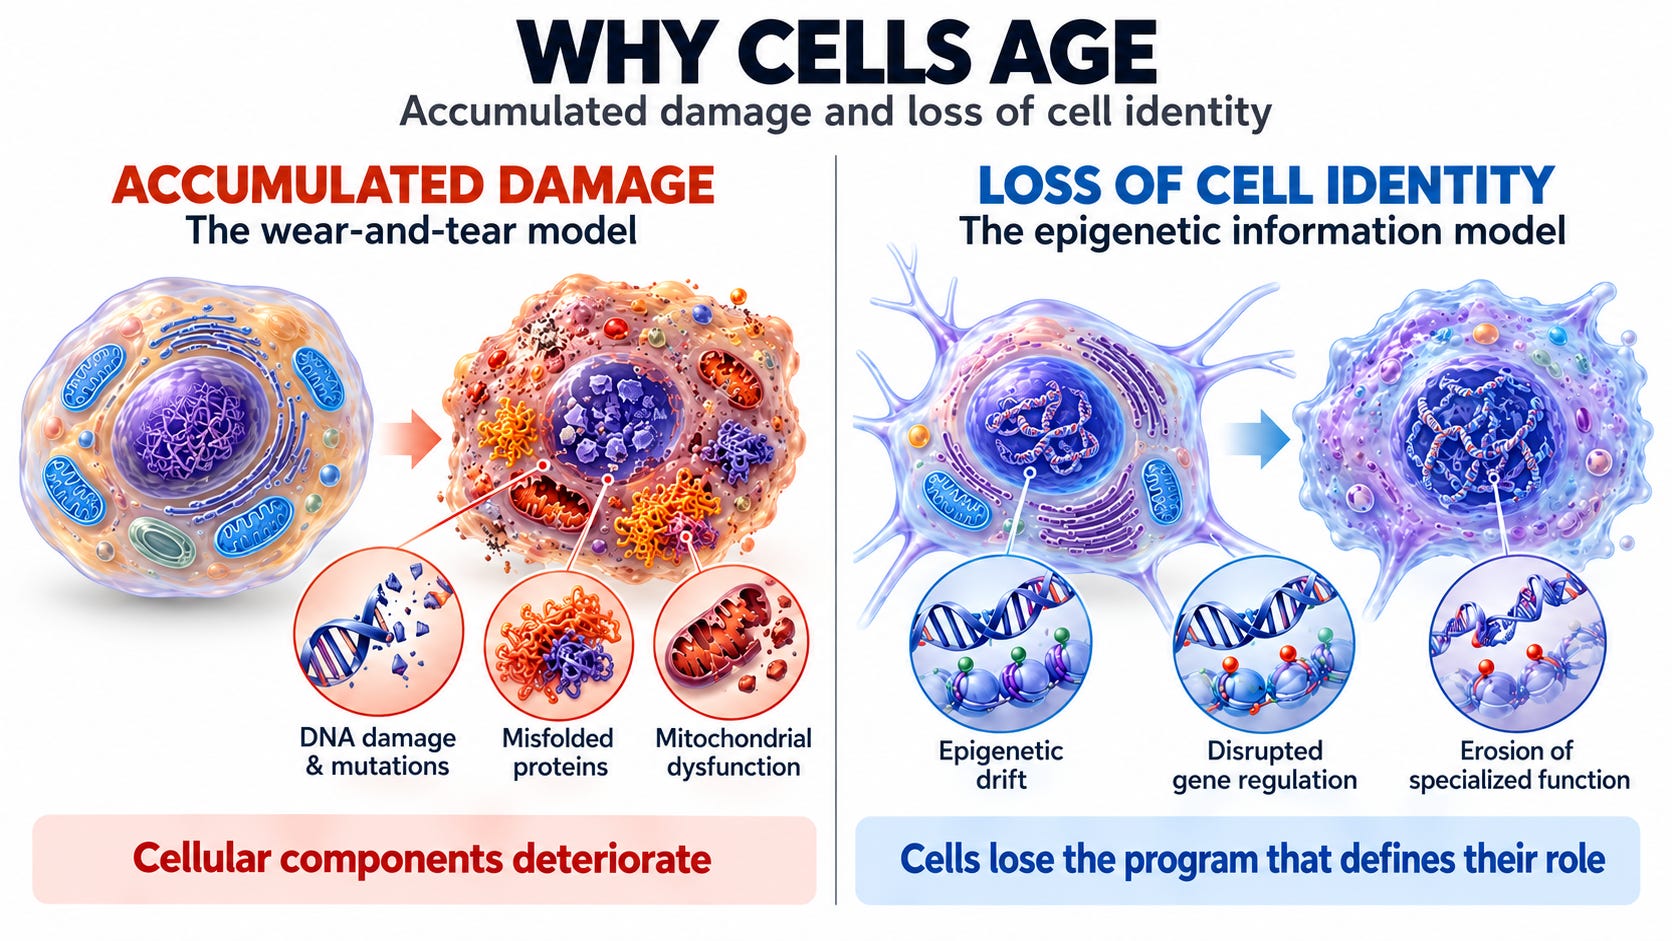
In this edition of Ground Truths I’m going to explain the loss of cell identity, how it leads to mesenchymal drift (fibrous scarring and inflammation), and how this new model furthers the potential to intervene in the aging process.
In embryonic and early development, our cells establish an identity. It’s locked in throughout our lives, except when it’s lost during the aging process. Although the DNA of every cell of our body is the same (or very close, if interested, see), the epigenetic structure, that includes methylation side chains, histones, nucleosomes and chromatin, is 3-dimensional and differs as a function of cell type. This is happening in the cell’s “mission control,” the nucleus. The epigenetic structure is the bedrock for our cell-specific identity.
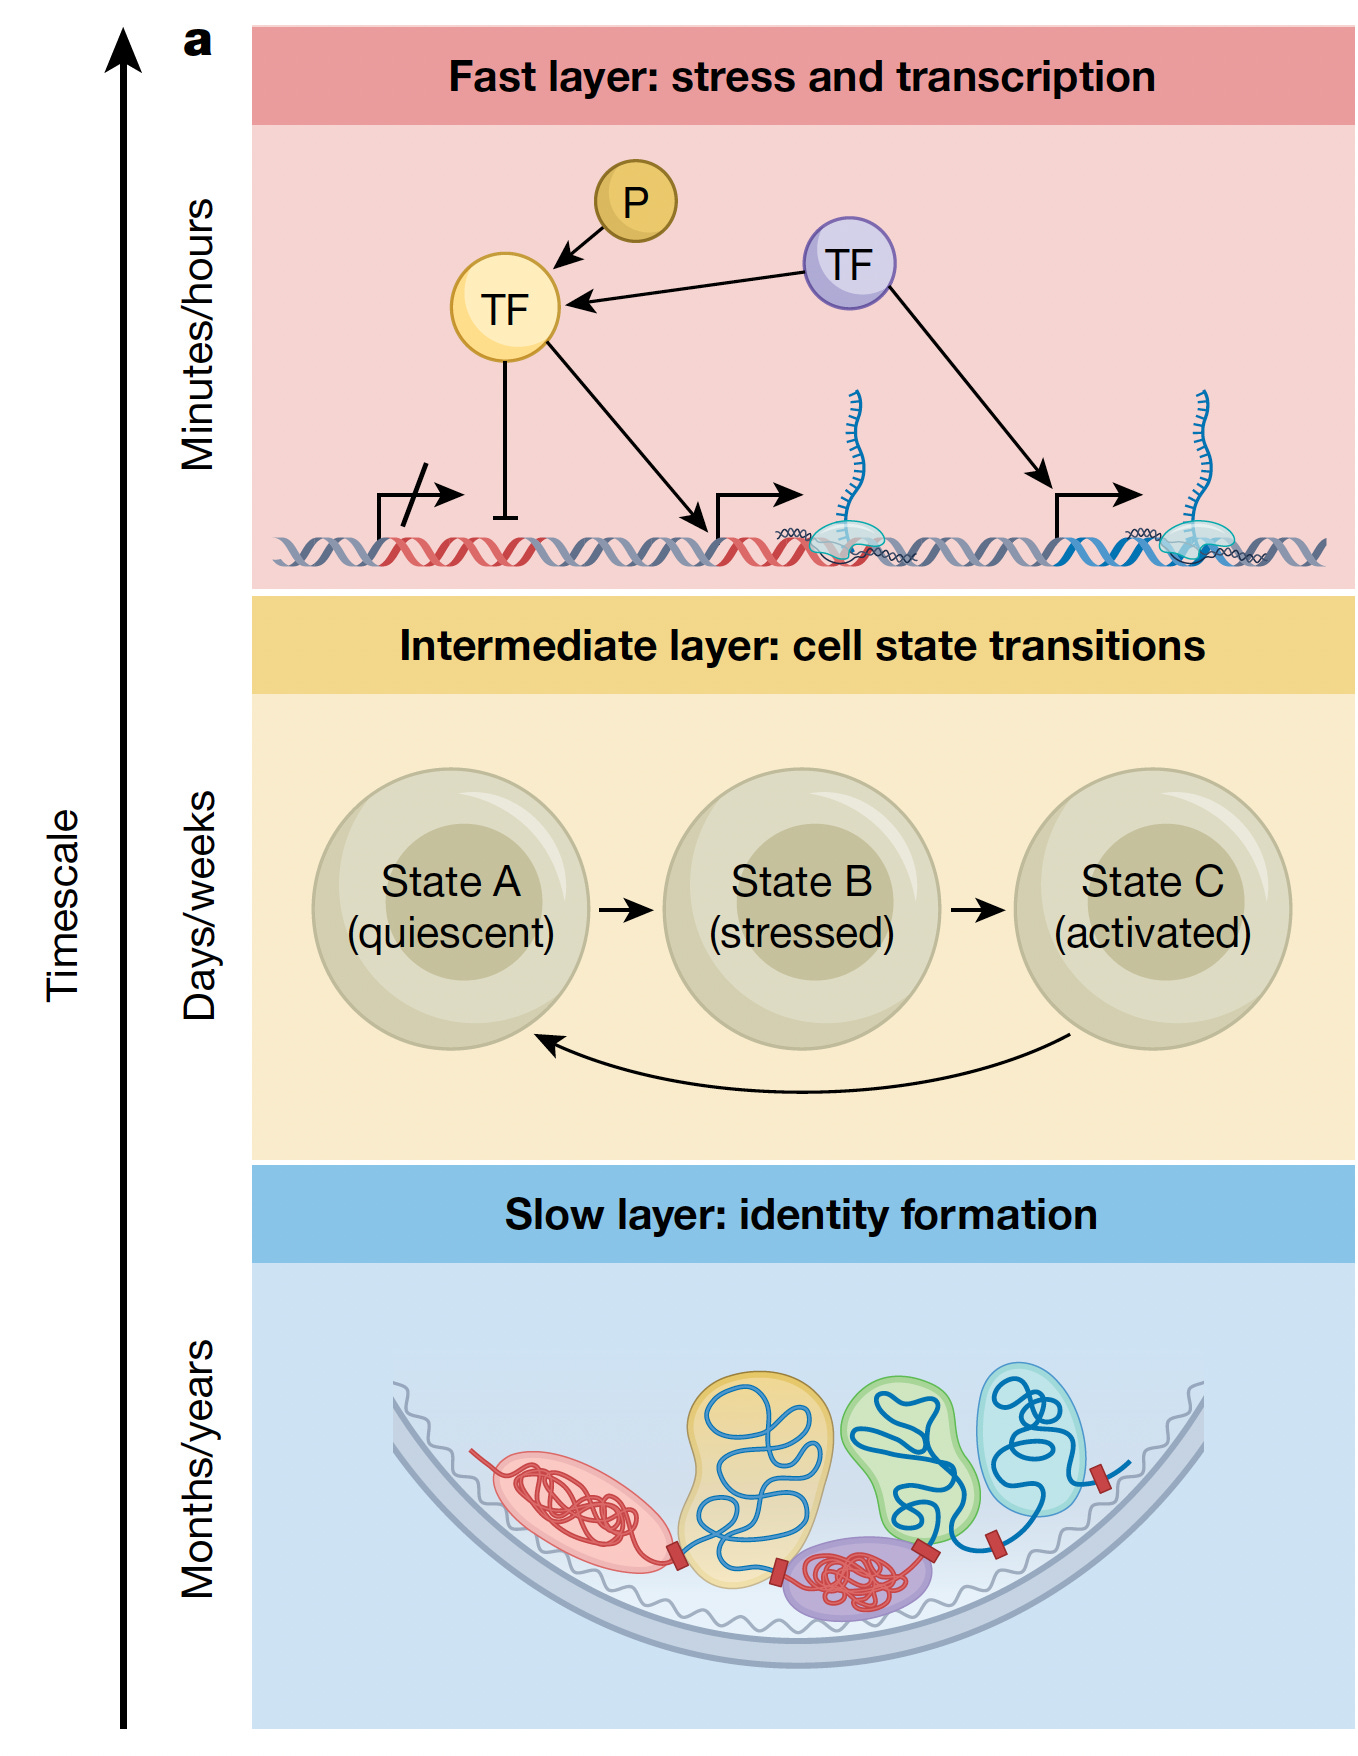
There’s a 3-tier regulatory “grammar” that maintains the cell identity as shown below.(Figure from the Nature paper). The fast layer responds to acute stress in a matter of minutes to hours and relies on production of transcription factors, like AP-1. The intermediate layer takes days to weeks to respond, going through cell state transitions such as activating a cell to promote healing and return to its basal state. The key is the slow layer, he one that locks and insulates the cell identity, the hard boundary, relying on chromatin architecture.
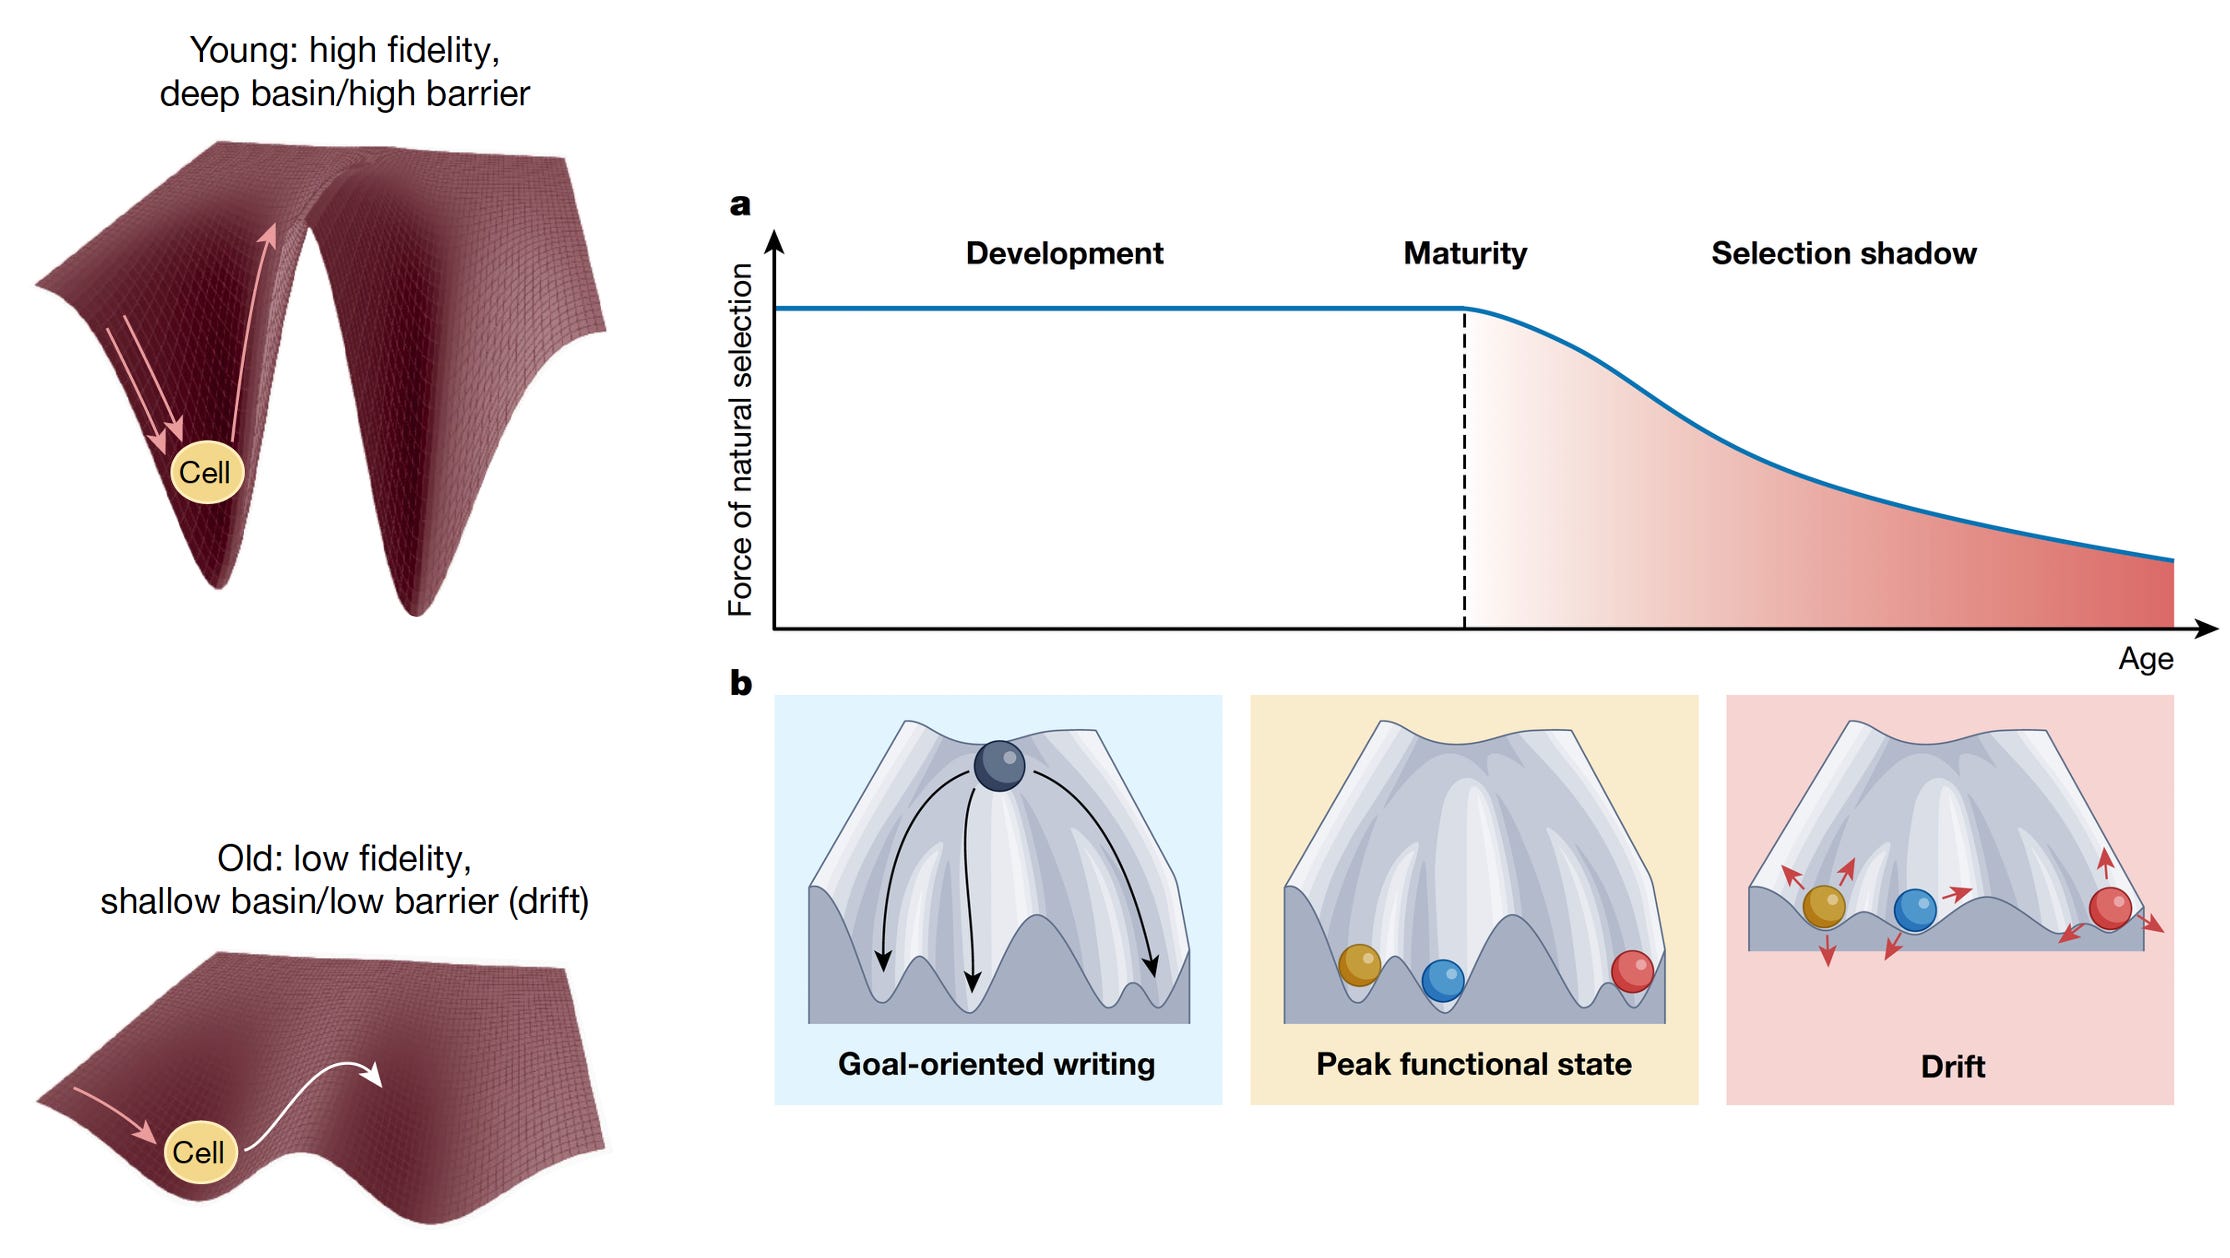
That gets us to Waddington’s epigenetic landscape model for how cells differentiate or de-differentiate, a model that has held up well from Conrad Waddington in 1957! A cell sitting down in the valley (Figure below, culled together from the Nature paper) represents a distinct specialized cell. The deep slope indicates the robustness, also called canalization, accompanied by a deep basin, maintains the identity of the cell, promotes its stability. The differentiated cell is “staying in its lane” in the landscape model and is constrained from sliding out, shifting identity. But with aging, the valleys lose their slope, the basin becomes shallow, there is loss of epigenetic constraints, and there is instability of cell identity. That sets up drift of cell identity, or what can be regarded as mesenchymal drift.
Over the lifespan, as shown on the right side of the Figure below, after peak maturation with the specialized cells (brain, liver heart,kidney, etc) fully and irrevocably differentiated (peak functional state below), the valleys are losing slope and the basins are progressively getting shallower, known as decanalization. The problem is that there is no evolutionary pressure to keep the grooves, valleys and basin in their youthful state, because the “selection shadow” is a post-reproductive trajectory.
The polycomb repressive complex 2 (PRC2) can be seen as the sculptor of this epigenetic landscape, the molecular machinery that shapes the grooves, valleys, and basin. It establishes the hard boundary, the deep epigenetic constraints for cell identity.
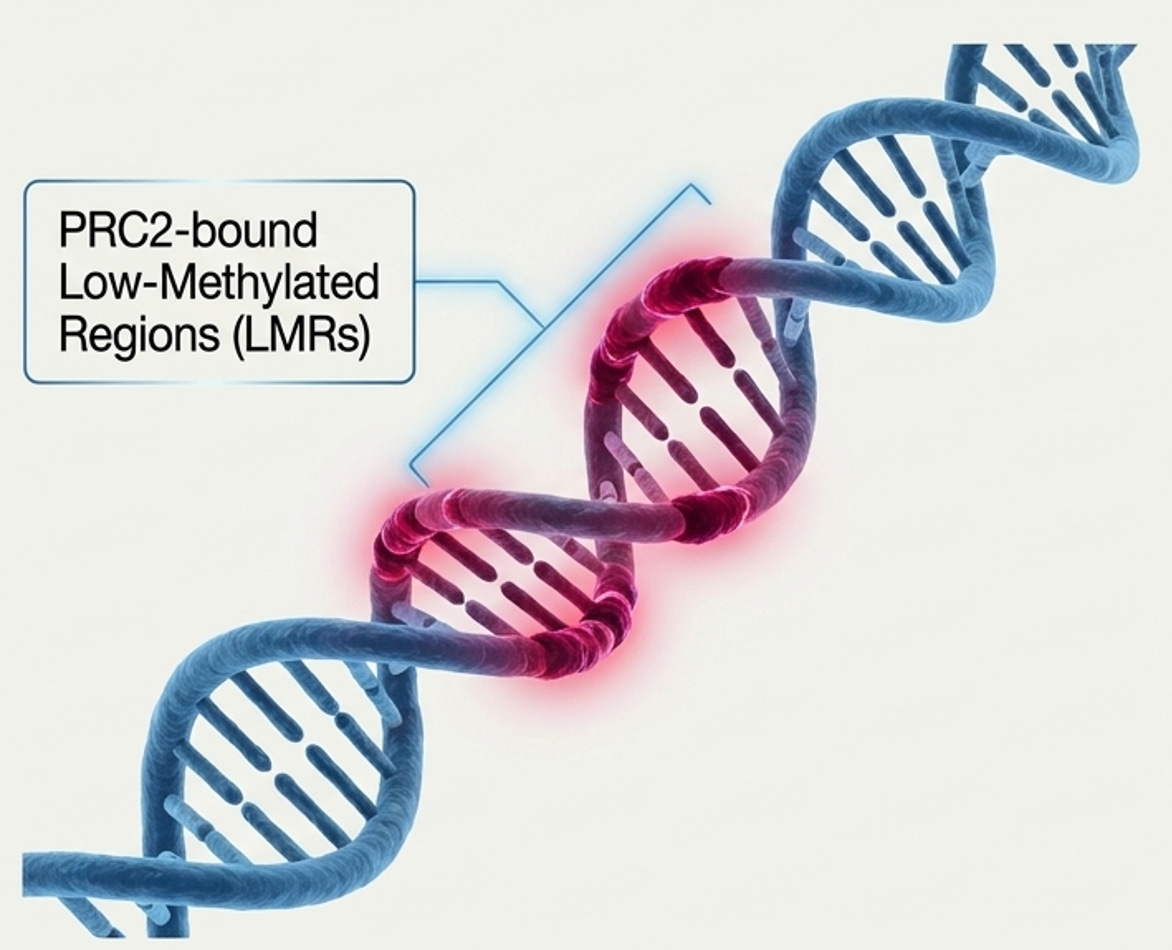
Epigenetic clocks are remarkably informative across 348 mammalian species, including humans, for predicting maximal lifespan and life history, but we didn’t know what they are actually measuring. It turns out it’s PRC2, the pace of slow layer erosion! (Figure below, to be precise, it’s the PRC2 low-methylated regions).
PRC2 comes into play when there is chronic inflammation overriding the fast layer capacity to respond and blocking PRC2, leading to erosion of the Waddington landscape, promoting cell identity loss. Even after chronic inflammation is resolved, there are epigenetic changes in chromatin that can persist. This loss of epigenetic grammar can also be the foundation for cancer cells. Eventual erosion of the slow layer essentially portends architectural collapse of the Waddington landscape.
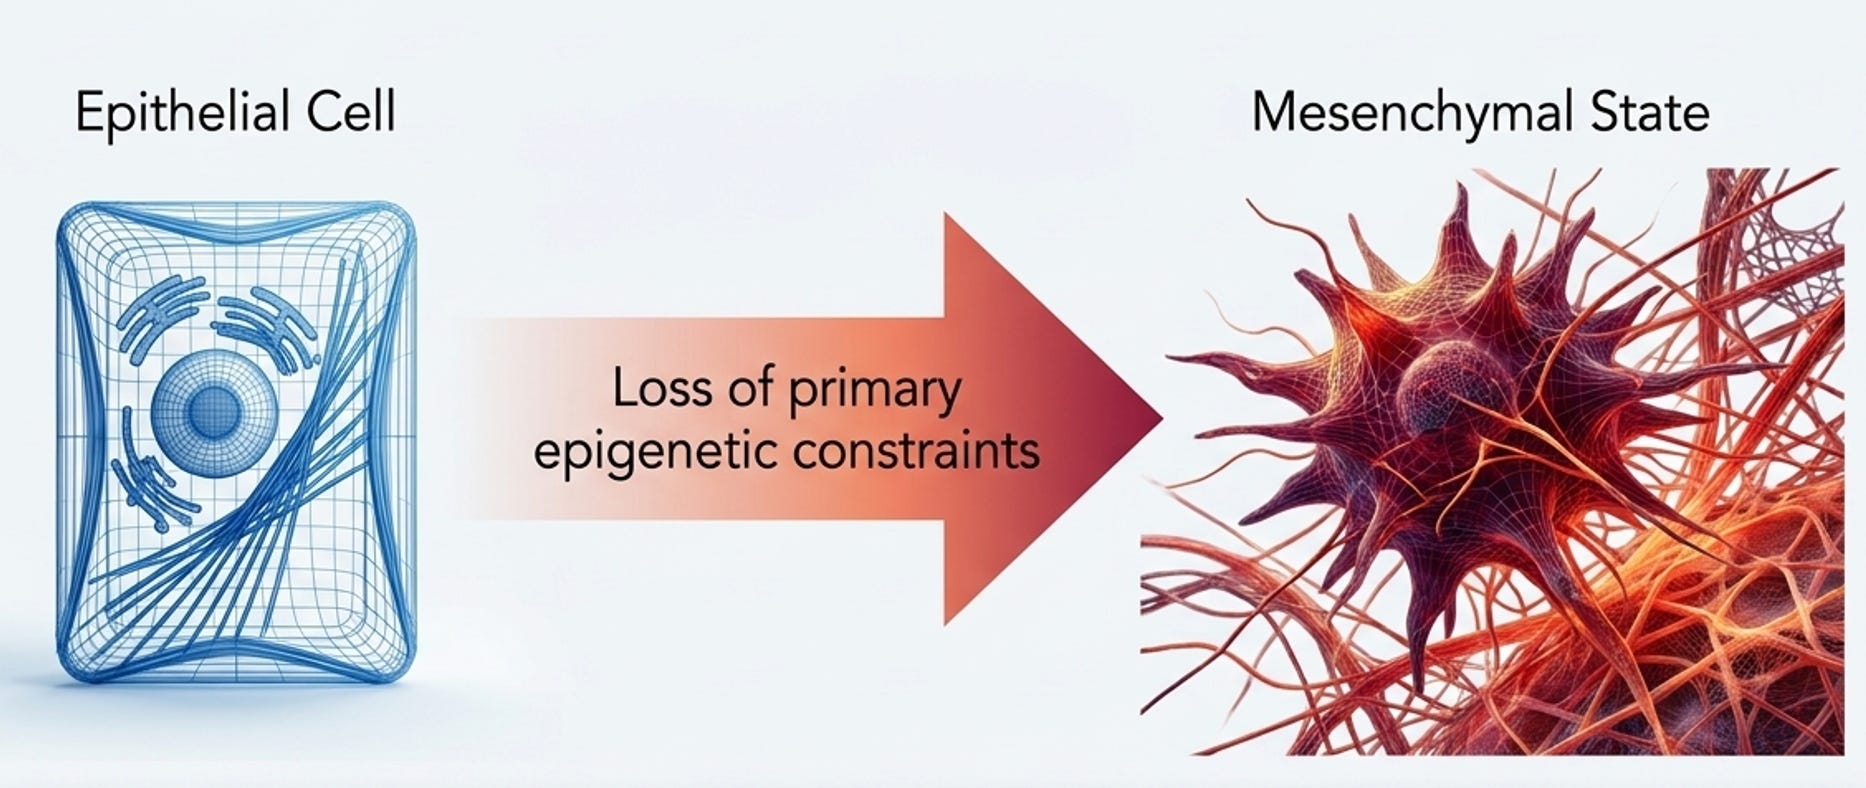
The mesenchymal state, as schematically shown below, in this example for an epithelial cell representative of all differentiated, specialized cells.
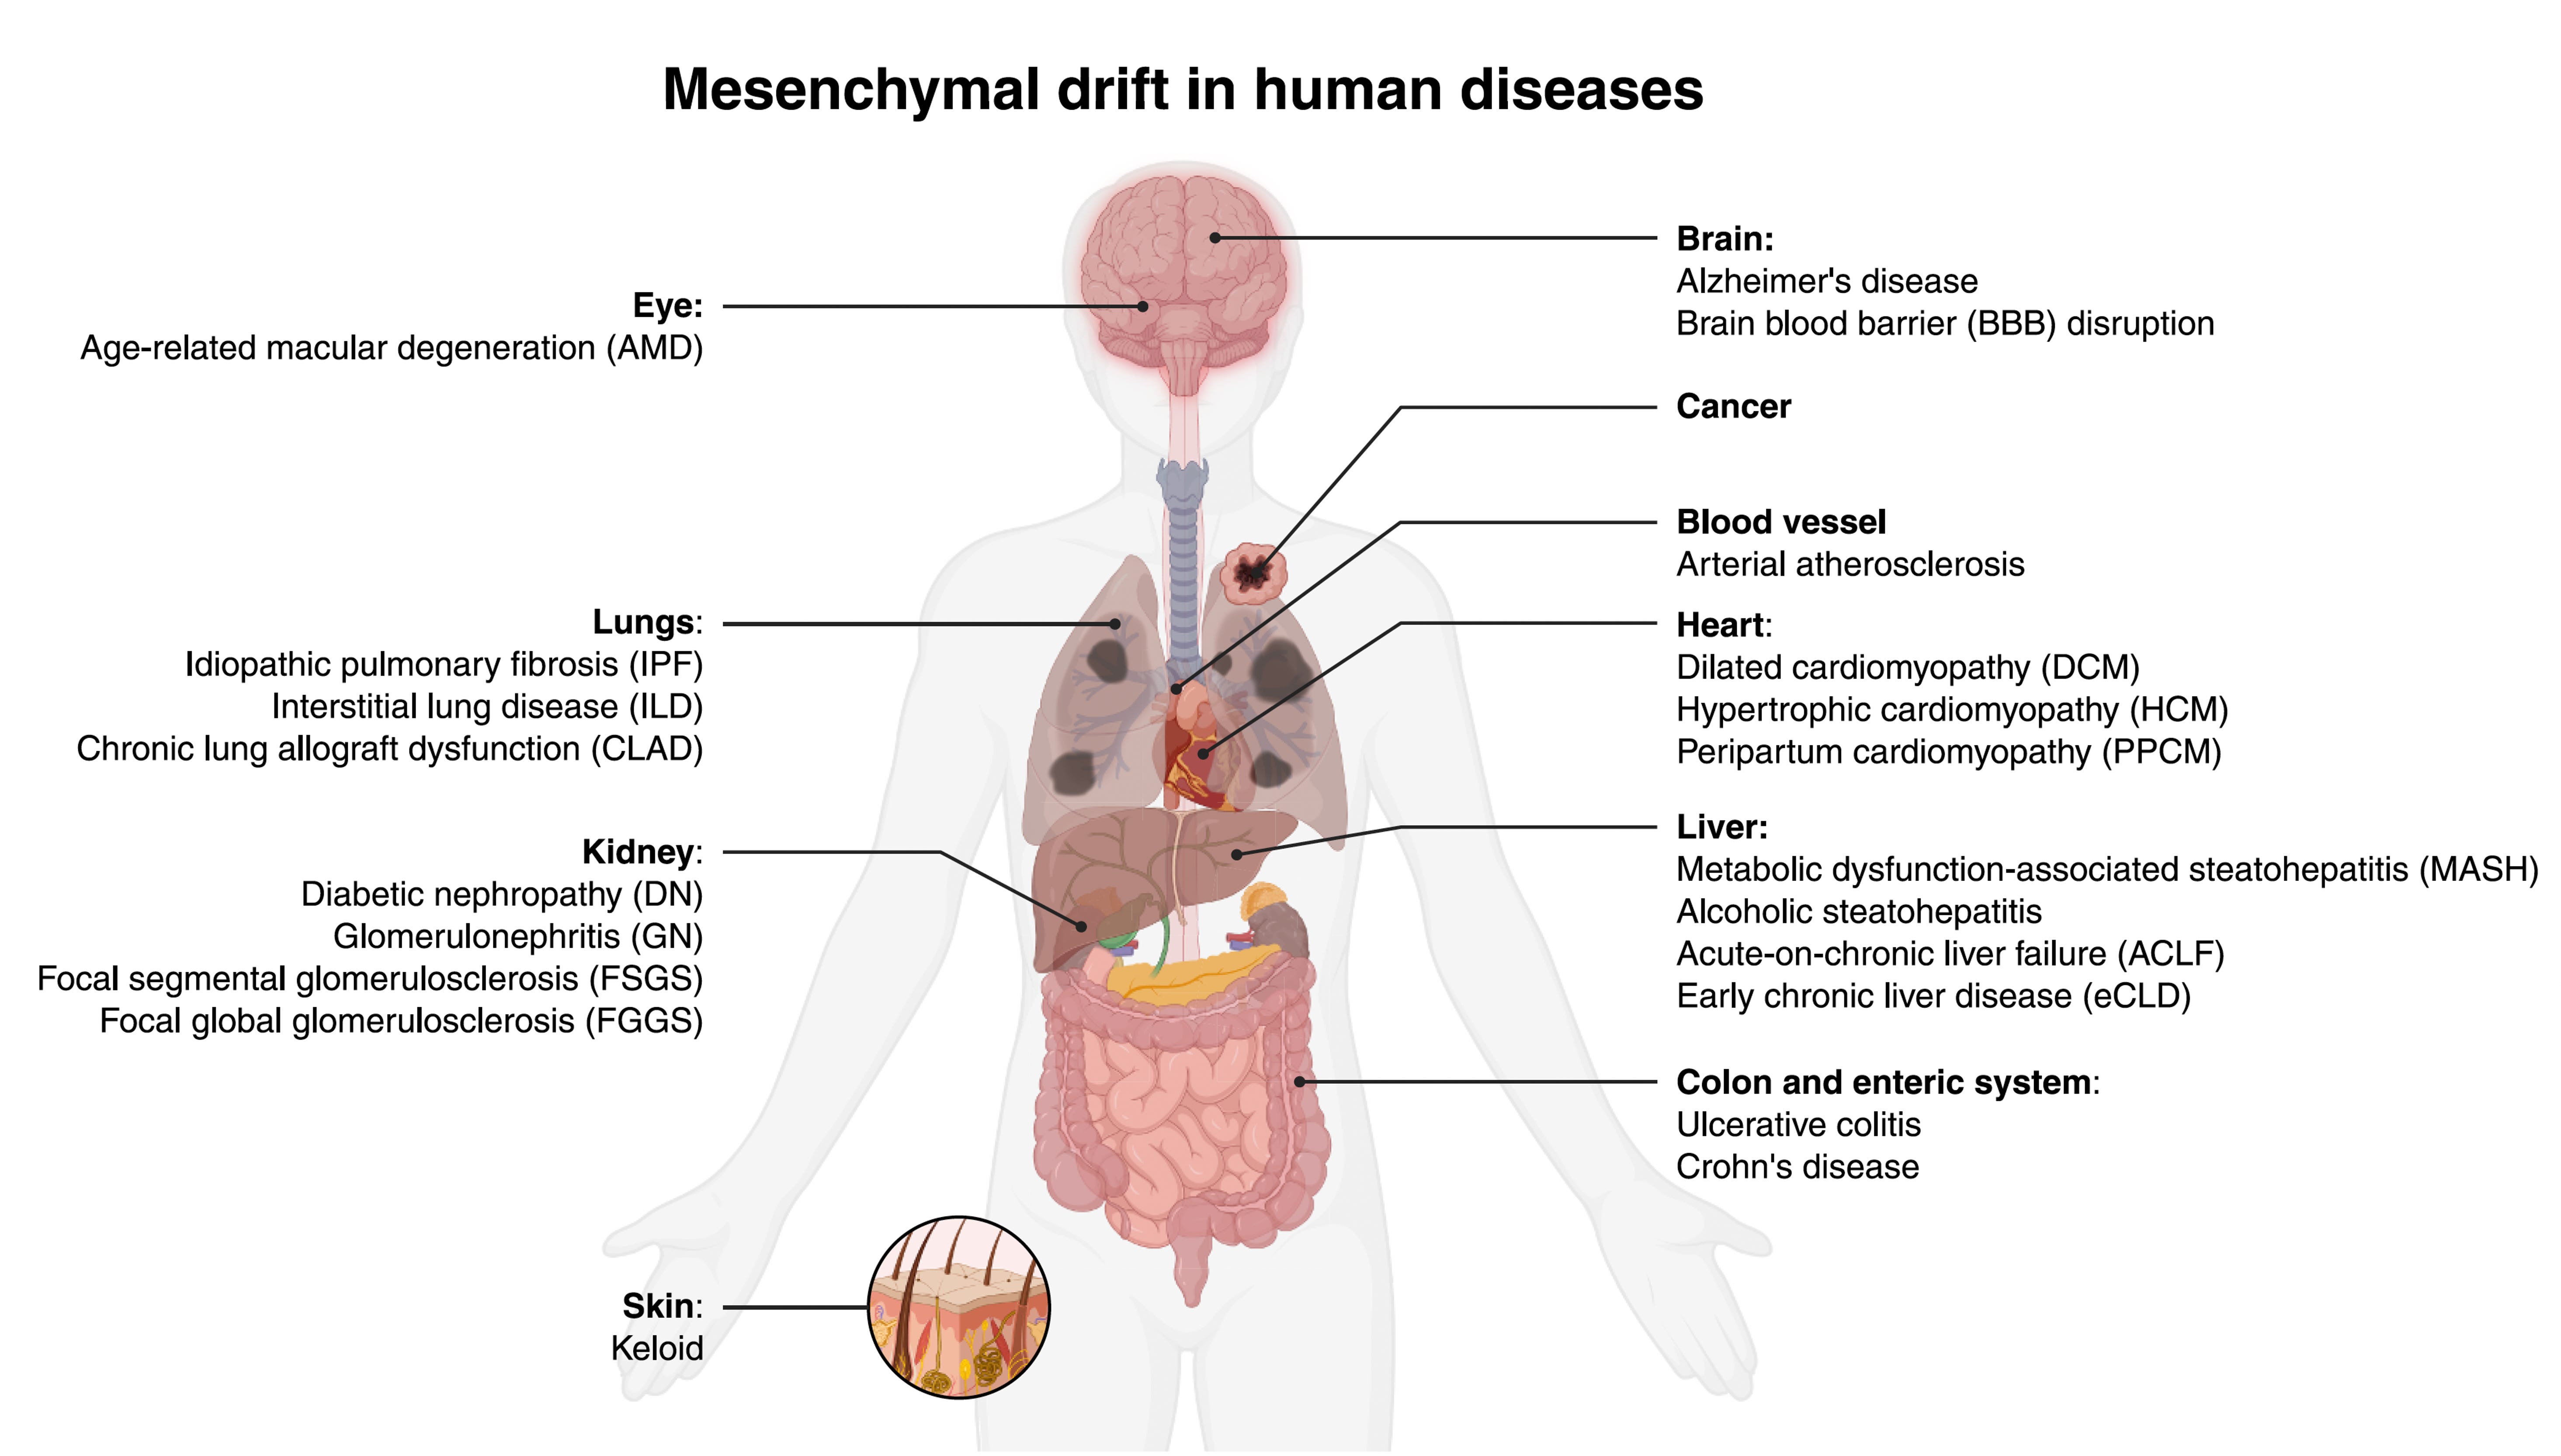
Now we turn to the Cell paper which goes deep on the mesenchymal drift. This denotes the change of cells to a mesenchymal state, resembling fibroblasts, engendering fibrous scar, laying down extracellular matrix, like mushy putty. It has been verified in 46 tissue types and is part and parcel of disease progression and poor outcomes, as shown below (Figure from the Cell paper). If you are checking for the tie-in between mesenchymal drift and age-related diseases, you’ll find them here, from atherosclerosis, to age-related macular degeneration, to Alzheimer’s disease.
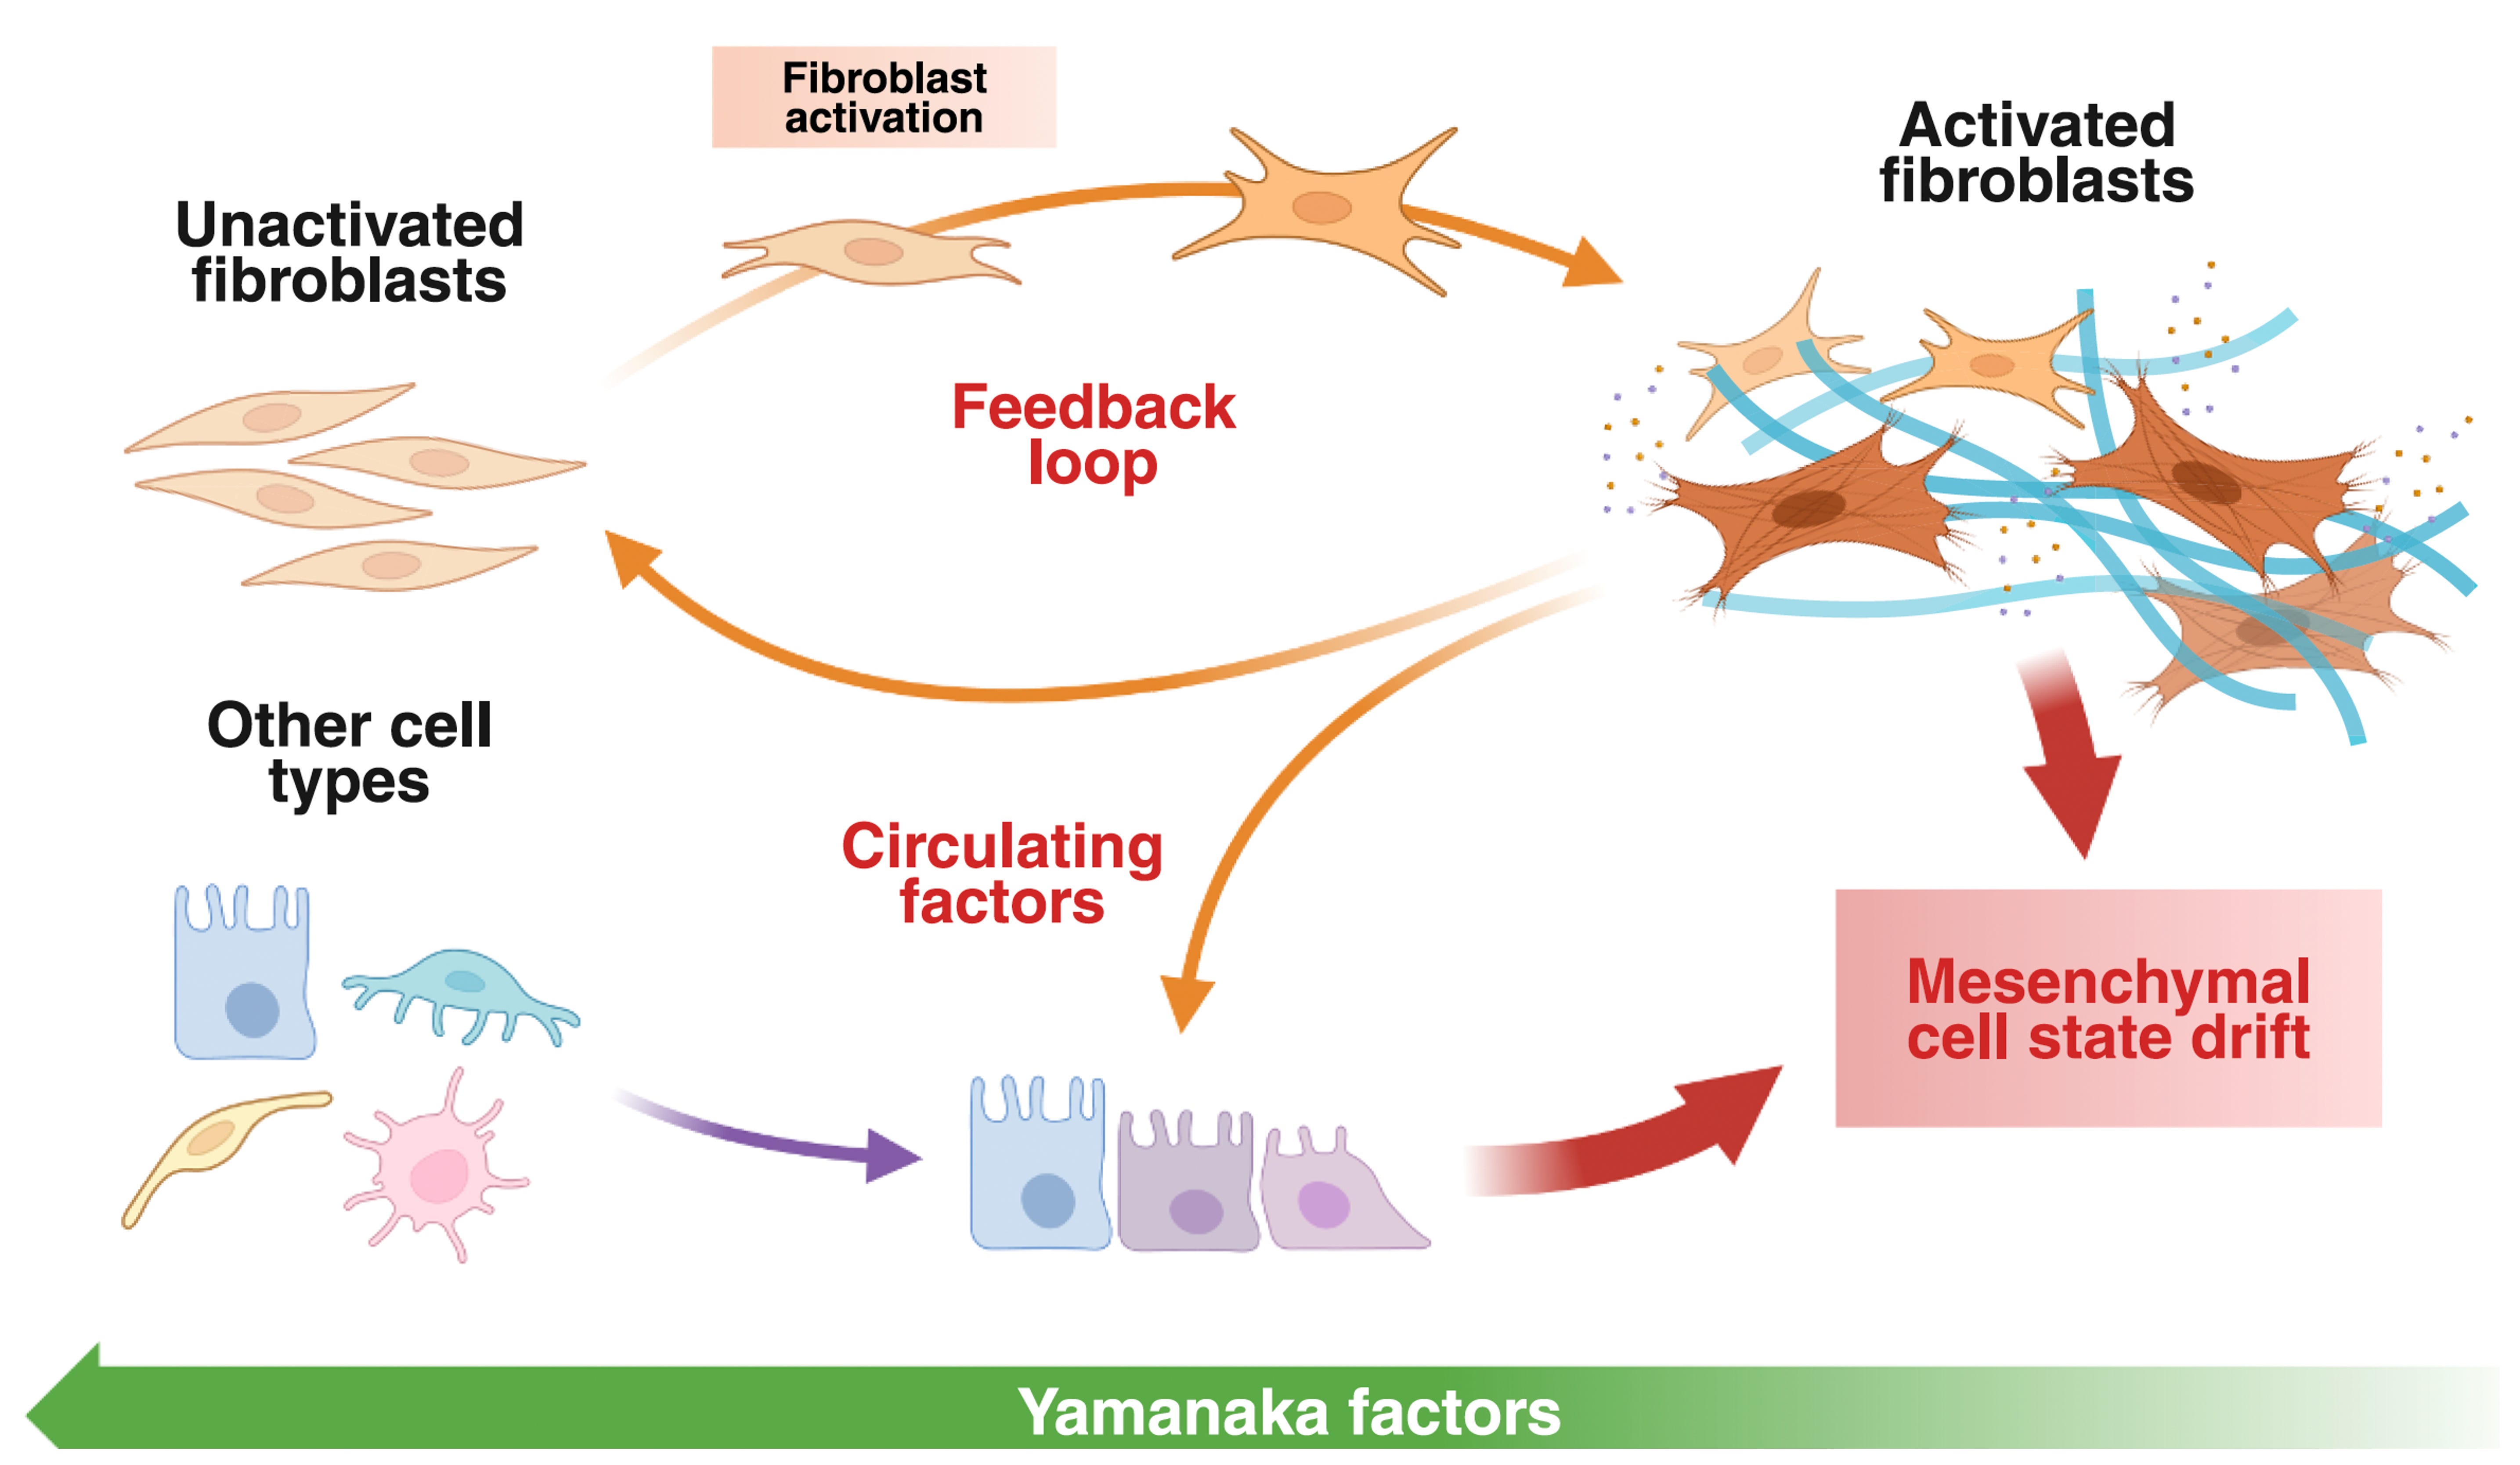
Now that we have an enhanced understanding of the process, which has a positive feedback loop as depicted below, fibroblast sthat are activating in turn activating more fibroblasts to induce scarring (Figure from the Cell paper), how can we intervene to freeze the drift, avoid the slow layer erosion, and preserve the Waddington landscape, keeping cells locked in their designated identity? Or, even more ambitious, actually turn back the loss of erosion that has occurred?
Caloric restriction (CR), with its attendant reduced acetyl CoA, and reduced PRC2 methylation, promotes the preservation of slow layer architecture, conceptually freezing the drift. CR has been shown to promote lifespan in mammalian species but the results in non-human primates have been inconsistent, and the magnitude and duration of caloric restriction likely required in people is impractical. Still there may be, theoretically, a partial effect of avoidance of high caloric intake to help prevent erosion.
The use of the Yamanaka stem cell factors is the far-reaching intervention—rejuvenating cells— that has attracted the most attention and huge investment by biotech companies. But it’s tricky because it requires a brief exposure to the 4 transcription factors, OSKM (Oct-4, Sox2, Klf4, c-Myc), called “partial” epigenetic reprogramming, in order to avoid full reprogramming, which erases their memory and turns cells into pluripotent stem cells. That carries an increased risk for cancer. But partial reprogramming using short bursts, rejuvenation is seen, with restoration of cell identity in aged human fibroblasts (even from age 96 years) and in animal models. The slow layer is restored, the PRC2 domains are re-established, and the mesenchymal drift is actively reversed. An alternative to short exposure for partial reprogramming is the use of 3 transcription factors OSK (no c-Myc) which is being tested in a pilot study of patients with severe optic nerve damage using direct eye injection.
The Nature paper also gets into lithium as an intervention for maintaining neuron identity by interfering with the pathway of slow layer failure. I won’t get into the details of all the mediators (β-catenin, EDH2-USP7, KDM1A, REST, GSK3β, etc) but lithium’s impact on GSK3β blocks tau phosphorylation in experimental models. Lithium orotate has been raised as a candidate for preventing Alzheimer’s, as I’ve previously written about, and this mechanism may be operative.
There continues to be extraordinary progress in the science of aging. Beyond the old dogma that this is just the cumulative outgrowth of cell mutations and damage, we now understand the epigenetic basis: the loss of cell identity serves as both a driver and result of the aging process. The basic 3-tiered grammar is understood, as are the potential interventions to freeze the mesenchymal drift or directly restore (“rejuvenate”) cell identity. Whether the latter will be capable of safely bringing back the Waddington landscape and reverse aging in humans at the wheel body, organ, or tissue level, remains uncertain.
But we know that chronically stressing the fast layer can be detrimental for the integrity of the essential slow layer. It follows that lifestyle factors, like a pro-inflammatory diet, lack of exercise, or poor sleep quality, can be viewed as chronic stressors that could promote the slow layer erosion and accelerate the loss of cell identity.
The mesenchymal drift story, a fibroblast-like takeover due to loss of cell identity, is exceedingly important as an explanation for the incidence and progression of so many diseases. Slippage of identity can lay the foundation for a cell to become cancerous, yet another bad sequelae. Undoubtedly, loss of cell identity is a major underpinning of age-related diseases.
I was frankly surprised that the new Nature paper did not cite the prior Cell one, since the refined model had much of its basis previously described. Perhaps that was a simple oversight. If there is more interest in partial epigenetic reprogramming, I recommend 2 prior papers (here and here).
One practical takeaway from this work is finally knowing what the epigenetic clock is measuring. I interviewed Steven Horvath, the pioneer of epigenetic clocks when, not very long ago, it was unclear what information was being captured and how these clocks were so accurate. Now it is.
I have purposely omitted many details in this post to not lose the reader. That oversimplification may be disturbing to the epigeneticists. On the other hand, others will say this was above their head. It’s always hard to strike the right balance, especially for a complex topic like this, but I hope you found it helpful. If we are going to slow our aging process and extend our healthspan, understanding the biology will be essential.
NB. I wrote this post. No AI. I did use AI to generate three of the Figures as noted above to help the reader visualize what I was writing about. I have no conflicts of interest related to this topic or post.
Ground Truths has 217,000 subscribers from every US state and 214 countries. There are over 300,000 followers of Ground Truths so more than 100,000 folks who can easily convert to be free subscribers.
Your subscription to these free essays and podcasts makes my work in putting them together worthwhile. If you’re not a subscriber, please join!
If you found this interesting PLEASE share it!
The proceeds from all voluntary paid subscriptions go to support our summer internship program. It enabled us to accept and support a record number of 62 summer interns that joined us in 2026! These are high school, college and medical students selected from thousands of applicants. We couldn’t do this expanded program without the funds coming in through Ground Truths. Thank you!